The dinoceratans were a lineage of hoofed herbivorous mammals whose evolutionary affinities are a little uncertain, but may have been related to the South American meridiungulates. Found in Asia and North America from the late Paleocene to the late Eocene, they had bulky rhino-like bodies and were some of the largest terrestrial animals of their time.
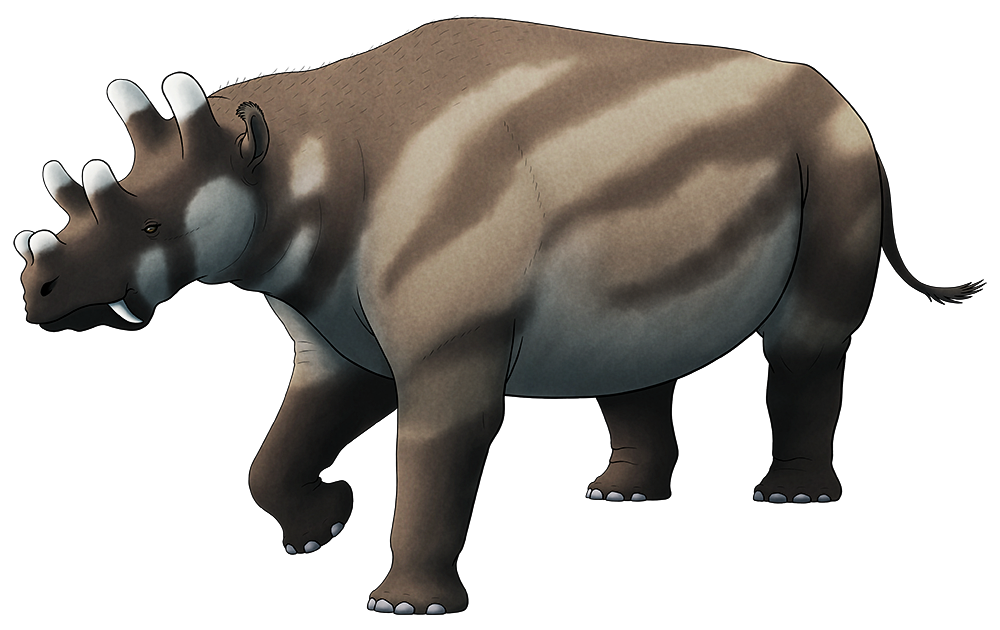
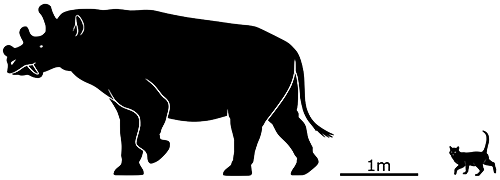
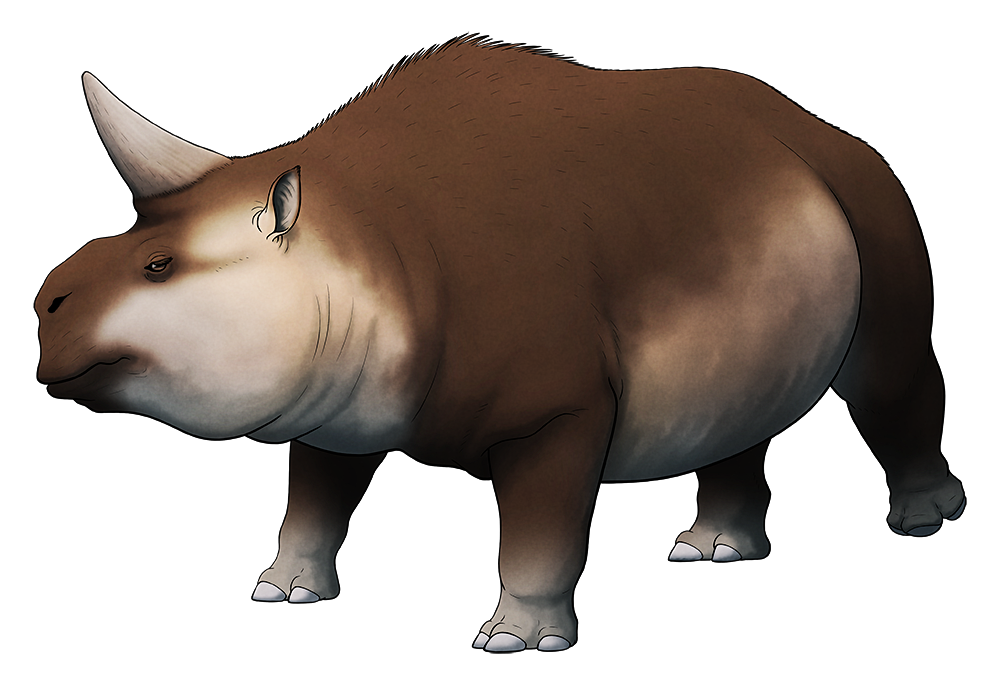
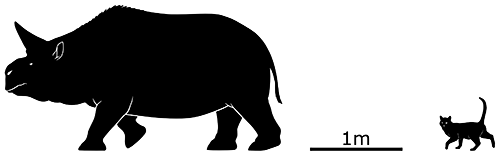
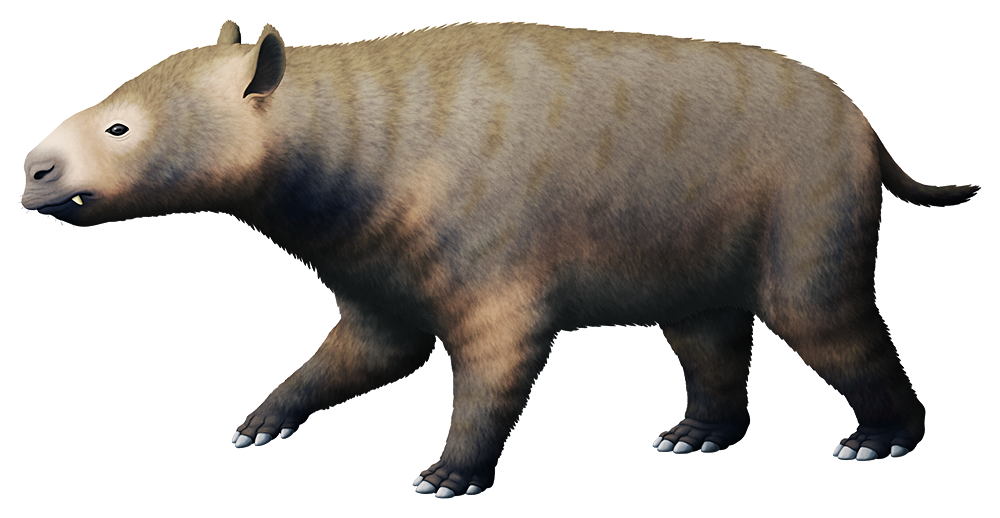
Eobasileus cornutus was one of the biggest of them all, measuring around 2.1m tall at the shoulder (~7′) and living in the Western United States during the early Eocene, about 46-40 million years ago.
And it had a very odd-looking head, with six blunt ossicone-like horns, large sabre-like fangs, bony flanges on its lower jaw, a concave forehead, and a proportionally tiny brain for its body size. The horns and fangs were sexually dimorphic, much smaller in females, suggesting they were mainly used for display or combat between males.
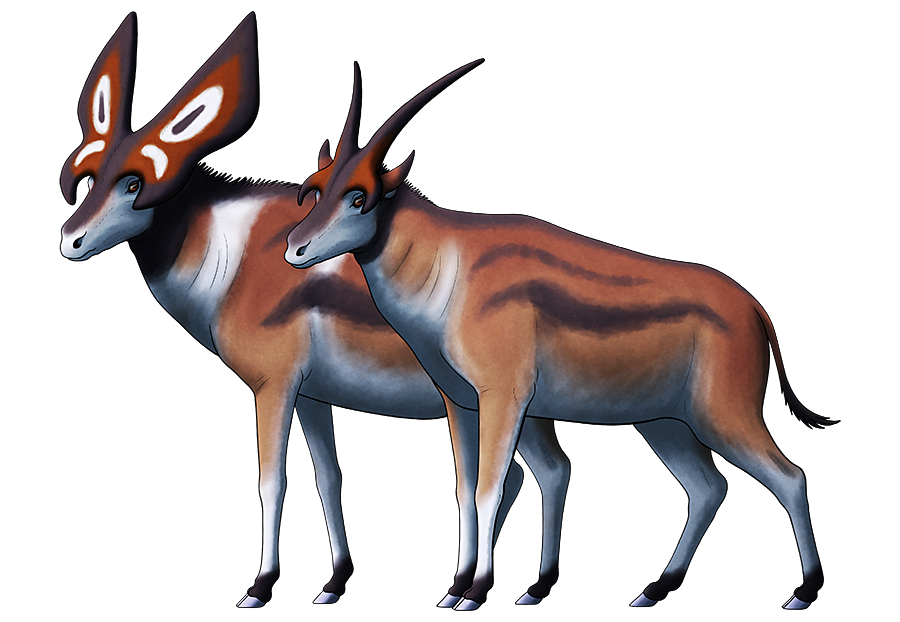
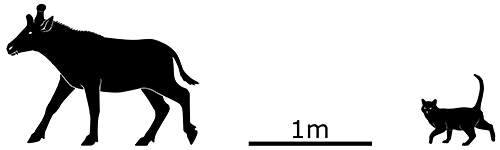
And Prolibytherium was probably the most striking of the lot.
Two different species have been identified, with Prolibytherium magnieri here living in North Africa during the early-to-mid Miocene, about 17-16 million years ago. Its exact evolutionary relationships are uncertain but it was probably part of a group called climacoceratids, deer-like giraffoids which often had thorny branching ossicones that resembled antlers.
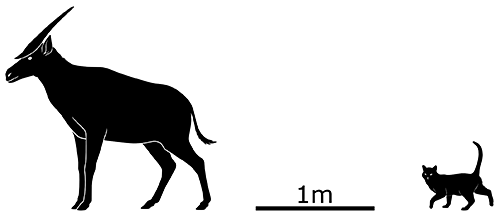
It stood around 1.2m tall at the shoulder (~4′), and exhibited dramatic sexual dimorphism – females had slender forked horn-like ossicones, while those of the males flared out into large wide flat shapes that resembled butterfly wings.
Heavy reinforcement in the bones of the back of the males’ skulls helped to support all the extra weight of those huge ossicones, and if they actually used the structures to fight with each other then this may have also provided some protection or shock absorption.
Modern ruminants are the only living mammals with bony headgear, with four different lineages each sporting a slightly different type: deer antlers, bovid horns, giraffid ossicones, and the prongs of pronghorns.
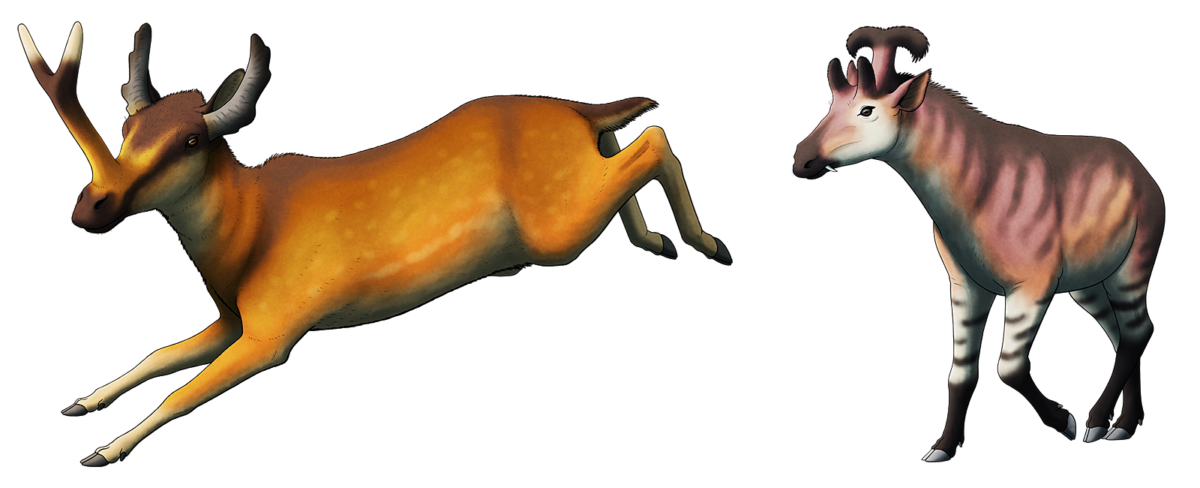
The protoceratids were an early group of North American ruminants whose relationships are uncertain, but may have been related to modern chevrotains. They were convergently deer-like in appearance, with teeth adapted for grazing on tough grasses – and along with having a pair of horns in the usual position on their heads, males also sported an additional pair of ossicone-like growths on their noses.
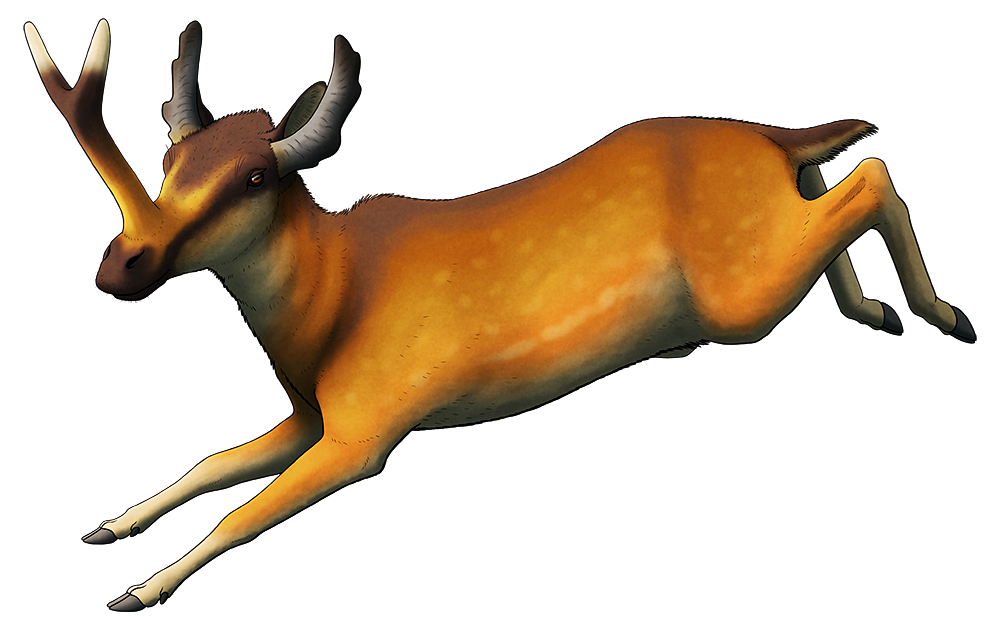
Synthetoceras tricornatus lived during the Late Miocene, around 10-5 million years ago, and was one of the largest protoceratids, standing about 1.1m tall at the shoulder (3’7″). Its two nose-horns were partially fused into a single long structure with a forked tip, which may have been used for sparring in a similar manner to the antlers of modern deer.
Synthetoceras tricornatus
Meanwhile on a different branch of the ruminant family tree, closer related to deer and giraffes, a group known as the palaeomerycids independently developed a similar sort of extra head appendage – but at the opposite end of their skulls.
These ruminants were a little more heavily built than the protoceratids, and specialized in feeding on soft vegetation in humid forest environments. They were a highly successful group, existing for almost 30 million years, ranging across Eurasia, Africa, and North America, and even ventured into South America during the early phases of the Great American Interchange.
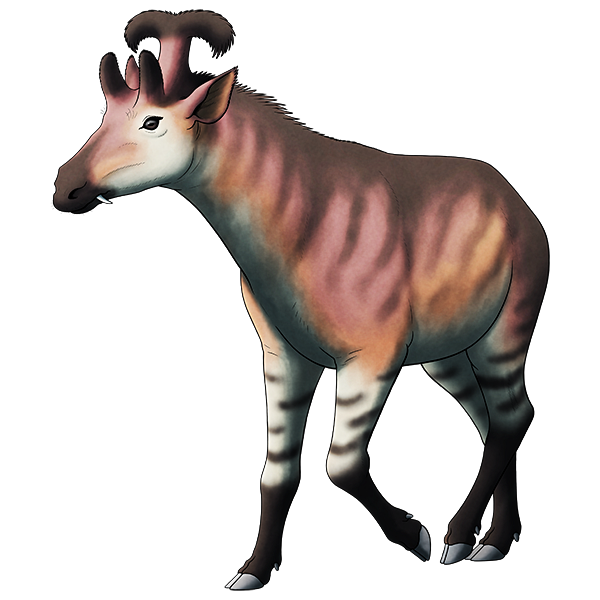
Males had two giraffe-like ossicones above their eyes, along with a third crest-like one at the very back of their heads. In some species this formed a single central “horn” shape, while in others it forked out to each side. They also often had long saber-like canine teeth similar to modern water deer and musk deer, which were probably used for fighting while their elaborate headgear was purely for visual display.
Xenokeryx amidalae lived in Spain during the mid Miocene, about 16 million years ago. It stood around 0.8-1m tall at the shoulder (2’7″-3’3″) and had a unique T-shaped “handlebar” crest which ended up inspiring its genus name – a reference to the similar shape of one of Queen Amidala’s headpieces in Star Wars, which was itself based on Mongolian imperial fashion.
South America was an isolated “island continent” for a large chunk of the Cenozoic, and during that time it was home to a unique mix of species evolving completely separately to the rest of the world.
And, like rhinos, some of them may even have had horns.
Hoffstetterius imperator lived in Bolivia during the late Miocene, about 11-5 million years ago. Standing around 1.6m tall at the shoulder (5’3″), it had a particularly oddly-shaped skull, with a deep downward-flaring lower jaw and a large bulging bony “shield” on its forehead that resembles the attachment points for horns on rhino skulls.
Keratinous structures like that only fossilize very rarely, so the actual size and shape of whatever attached there is unknown – the pointed horn shown here is one possibility – but we honestly don’t know what was going on with these guys’ heads.
We have a fairly good picture of the evolutionary origins of most groups of aquatic mammals – except for the pinnipeds. The fossil record of early seals is still rather sparse, and for a long time the earliest known species was Enaliarctos, an animal that was already very seal-like and didn’t help much in figuring out whether seals’ closest living relatives are bears or musteloids.
But then Puijila darwini was found in the late 2000s, a transitional form with a near-complete skeleton, filling in a gap in our understanding so conveniently it almost seems too good to be true.
Discovered in Nunavut, Canada, Puijila dates to the early Miocene, about 23-20 million years ago. It was a small freshwater otter-like animal, about 1m long (3’3″), with a long tail and webbed feet adapted for paddling with all four of its limbs.
It lived at around the same time as the more specialized Enaliarctos, so it wasn’t a direct ancestor of modern seals, instead being part of an early offshoot lineage that retained more basal characteristics – but it does gives us a clue as to what the earliest pinnipeds looked like. Along with genetic studies it also helped to clarify that seals’ closest relatives are indeed the musteloids, although they’re estimated to have last shared a common ancestor around 45 million years ago so there’s still a lot of time unaccounted for in the proto-seal fossil record.
Several other fossil species that were previously thought to be musteloids have now also been recognized as close relatives of Puijila, and it seems that they were a fairly widespread group basically filling the ecological niche of otters at a time before true otters existed.
Most surprising and frustrating of all, however, is that some of these other otter-seals actually survived all the way into the Pleistocene, only going completely extinct sometime in the last 2 million years.
The earliest baleen whales didn’t actually have any baleen plates in their mouths, and the evolutionary origin of these unique filter-feeding structures is still poorly understood.
It was thought to have been a fairly simple linear process from toothed ancestors to a mix of teeth and baleen and then to fully toothless with just baleen, but more recent discoveries have begun to cast doubt on that idea. The teeth of ancestral baleen whales weren’t suited to filter-feeding at all, instead still being adapted for predatory piercing and chewing – actions which would have been constantly interfering with and damaging any proto-baleen forming alongside them, and making it seem much more unlikely that there would have ever been a transitional form that had both teeth and baleen at the same time.
But then how did baleen whales get their baleen?
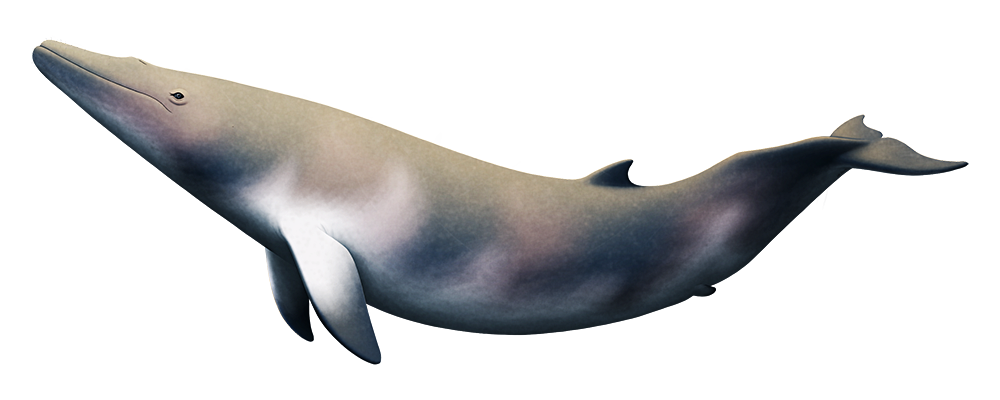
Maiabalaena nesbittae here provides a possible solution. Discovered in Oregon, USA, this early baleen whale dates to the early Oligocene, around 33 million years ago, and compared to most of its modern relatives it was comparatively tiny, only about 4.6m long (15′).
And it had no teeth at all, but possibly also no baleen.
Baleen rarely fossilizes, so it’s unclear whether Maiabalaena actually had any or not, but the shape of its skull suggests it probably didn’t – it lacked the broad thickened upper jaw associated with supporting racks of baleen plates. It instead seems to have been adapted for suction feeding similar to modern belugas and beaked whales, using muscular cheeks and tongue to manipulate water pressure and pull small prey like fish and squid straight into its mouth.
Since it lived at a time when the Antarctic Circumpolar Current was forming and cooling the oceans, changing ecosystems and prey availability, it may represent a previously unknown stage in baleen whale evolution – a point when they’d moved towards specializing for suction feeding and lost their teeth entirely, before transitioning again over to filter-feeding with baleen in a completely separate evolutionary development a few million years later.
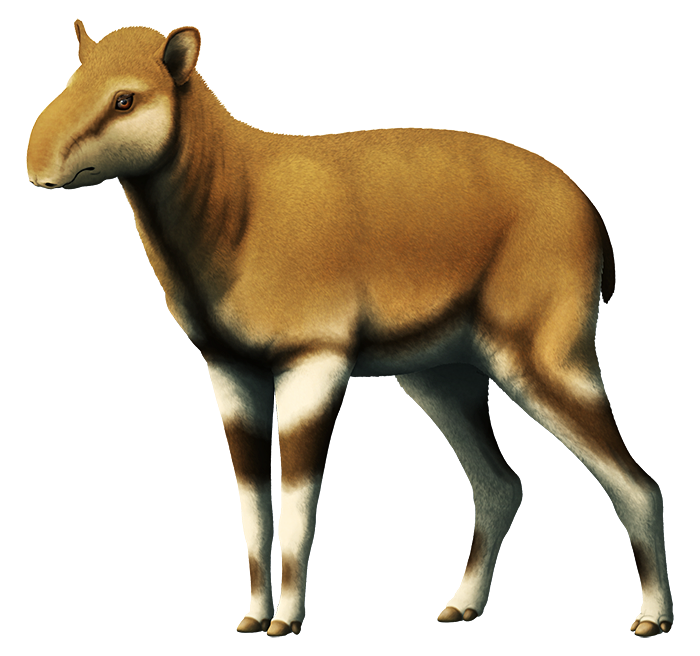
Lophialetes expeditus was one of these odd tapir-relatives, living in Mongolia and China during the mid-Eocene about 48-37 million years ago. Standing around 50cm tall at the shoulder (1’8″) it had a build more resembling a deer or a horse than its pig-like modern cousins, and it was adapted for fast running in open plains, with long slender legs and three-toed hoofed feet that bore most of its weight on the middle digit.
Its skull had a nasal region similar to both modern tapirs and saiga antelope, suggesting the presence of a short trunk-like nose – but since some of its closest relatives didn’t have nearly such well-developed snouts, it seems that Lophialetes evolved its trunk separately to modern tapirs.
The modern sperm whale is already an impressive animal, being by far the largest of the living toothed whales and famous for its ability to dive over 2km down (1.2 miles) to feed on deep-sea animals like giant squid.
But some of its ancient relatives were terrifying.
Livyatan melvillei here has an appropriately monstrous name, inspired by both the Hebrew name for the Leviathan and Herman Melville, the author of Moby-Dick. Known from the Pacific coast of South America during the late Miocene, around 10-9 million years ago, it’s estimated to have measured somewhere between 13.5m and 17.5m long (~44′-57′) – comparable in size to an adult male sperm whale.
Unlike the relatively slender mouth of its modern cousin, however, it instead had thick strong jaws full of enormous teeth.
It was part of a loose grouping of what are known as “macroraptorial sperm whales“, which all had similarly toothy jaws and occupied the same sort of ecological niche as modern orcas, specializing in hunting prey like large fish, squid, seals, and other whales.
Livyatan‘s main food source was probably smaller baleen whales about half its own size, and its only real competition for this prey was the equally huge megalodon shark that shared the same waters.
A huge fossil tooth found in Australia suggests that Livyatan or a very close relative of it survived at least into the early Pliocene, about 5 million years ago. Around this time a cooling climate and dwindling numbers of its preferred prey would have eventually made a population of such enormous apex predators unsustainable, and driven this “killer sperm whale” into extinction – probably around the same time megalodon disappeared, about 3.6 million years ago.